
17.7: Appendix G- For Further Study
- Page ID
- 121319
\( \newcommand{\vecs}[1]{\overset { \scriptstyle \rightharpoonup} {\mathbf{#1}} } \)
\( \newcommand{\vecd}[1]{\overset{-\!-\!\rightharpoonup}{\vphantom{a}\smash {#1}}} \)
\( \newcommand{\dsum}{\displaystyle\sum\limits} \)
\( \newcommand{\dint}{\displaystyle\int\limits} \)
\( \newcommand{\dlim}{\displaystyle\lim\limits} \)
\( \newcommand{\id}{\mathrm{id}}\) \( \newcommand{\Span}{\mathrm{span}}\)
( \newcommand{\kernel}{\mathrm{null}\,}\) \( \newcommand{\range}{\mathrm{range}\,}\)
\( \newcommand{\RealPart}{\mathrm{Re}}\) \( \newcommand{\ImaginaryPart}{\mathrm{Im}}\)
\( \newcommand{\Argument}{\mathrm{Arg}}\) \( \newcommand{\norm}[1]{\| #1 \|}\)
\( \newcommand{\inner}[2]{\langle #1, #2 \rangle}\)
\( \newcommand{\Span}{\mathrm{span}}\)
\( \newcommand{\id}{\mathrm{id}}\)
\( \newcommand{\Span}{\mathrm{span}}\)
\( \newcommand{\kernel}{\mathrm{null}\,}\)
\( \newcommand{\range}{\mathrm{range}\,}\)
\( \newcommand{\RealPart}{\mathrm{Re}}\)
\( \newcommand{\ImaginaryPart}{\mathrm{Im}}\)
\( \newcommand{\Argument}{\mathrm{Arg}}\)
\( \newcommand{\norm}[1]{\| #1 \|}\)
\( \newcommand{\inner}[2]{\langle #1, #2 \rangle}\)
\( \newcommand{\Span}{\mathrm{span}}\) \( \newcommand{\AA}{\unicode[.8,0]{x212B}}\)
\( \newcommand{\vectorA}[1]{\vec{#1}} % arrow\)
\( \newcommand{\vectorAt}[1]{\vec{\text{#1}}} % arrow\)
\( \newcommand{\vectorB}[1]{\overset { \scriptstyle \rightharpoonup} {\mathbf{#1}} } \)
\( \newcommand{\vectorC}[1]{\textbf{#1}} \)
\( \newcommand{\vectorD}[1]{\overrightarrow{#1}} \)
\( \newcommand{\vectorDt}[1]{\overrightarrow{\text{#1}}} \)
\( \newcommand{\vectE}[1]{\overset{-\!-\!\rightharpoonup}{\vphantom{a}\smash{\mathbf {#1}}}} \)
\( \newcommand{\vecs}[1]{\overset { \scriptstyle \rightharpoonup} {\mathbf{#1}} } \)
\(\newcommand{\longvect}{\overrightarrow}\)
\( \newcommand{\vecd}[1]{\overset{-\!-\!\rightharpoonup}{\vphantom{a}\smash {#1}}} \)
\(\newcommand{\avec}{\mathbf a}\) \(\newcommand{\bvec}{\mathbf b}\) \(\newcommand{\cvec}{\mathbf c}\) \(\newcommand{\dvec}{\mathbf d}\) \(\newcommand{\dtil}{\widetilde{\mathbf d}}\) \(\newcommand{\evec}{\mathbf e}\) \(\newcommand{\fvec}{\mathbf f}\) \(\newcommand{\nvec}{\mathbf n}\) \(\newcommand{\pvec}{\mathbf p}\) \(\newcommand{\qvec}{\mathbf q}\) \(\newcommand{\svec}{\mathbf s}\) \(\newcommand{\tvec}{\mathbf t}\) \(\newcommand{\uvec}{\mathbf u}\) \(\newcommand{\vvec}{\mathbf v}\) \(\newcommand{\wvec}{\mathbf w}\) \(\newcommand{\xvec}{\mathbf x}\) \(\newcommand{\yvec}{\mathbf y}\) \(\newcommand{\zvec}{\mathbf z}\) \(\newcommand{\rvec}{\mathbf r}\) \(\newcommand{\mvec}{\mathbf m}\) \(\newcommand{\zerovec}{\mathbf 0}\) \(\newcommand{\onevec}{\mathbf 1}\) \(\newcommand{\real}{\mathbb R}\) \(\newcommand{\twovec}[2]{\left[\begin{array}{r}#1 \\ #2 \end{array}\right]}\) \(\newcommand{\ctwovec}[2]{\left[\begin{array}{c}#1 \\ #2 \end{array}\right]}\) \(\newcommand{\threevec}[3]{\left[\begin{array}{r}#1 \\ #2 \\ #3 \end{array}\right]}\) \(\newcommand{\cthreevec}[3]{\left[\begin{array}{c}#1 \\ #2 \\ #3 \end{array}\right]}\) \(\newcommand{\fourvec}[4]{\left[\begin{array}{r}#1 \\ #2 \\ #3 \\ #4 \end{array}\right]}\) \(\newcommand{\cfourvec}[4]{\left[\begin{array}{c}#1 \\ #2 \\ #3 \\ #4 \end{array}\right]}\) \(\newcommand{\fivevec}[5]{\left[\begin{array}{r}#1 \\ #2 \\ #3 \\ #4 \\ #5 \\ \end{array}\right]}\) \(\newcommand{\cfivevec}[5]{\left[\begin{array}{c}#1 \\ #2 \\ #3 \\ #4 \\ #5 \\ \end{array}\right]}\) \(\newcommand{\mattwo}[4]{\left[\begin{array}{rr}#1 \amp #2 \\ #3 \amp #4 \\ \end{array}\right]}\) \(\newcommand{\laspan}[1]{\text{Span}\{#1\}}\) \(\newcommand{\bcal}{\cal B}\) \(\newcommand{\ccal}{\cal C}\) \(\newcommand{\scal}{\cal S}\) \(\newcommand{\wcal}{\cal W}\) \(\newcommand{\ecal}{\cal E}\) \(\newcommand{\coords}[2]{\left\{#1\right\}_{#2}}\) \(\newcommand{\gray}[1]{\color{gray}{#1}}\) \(\newcommand{\lgray}[1]{\color{lightgray}{#1}}\) \(\newcommand{\rank}{\operatorname{rank}}\) \(\newcommand{\row}{\text{Row}}\) \(\newcommand{\col}{\text{Col}}\) \(\renewcommand{\row}{\text{Row}}\) \(\newcommand{\nul}{\text{Nul}}\) \(\newcommand{\var}{\text{Var}}\) \(\newcommand{\corr}{\text{corr}}\) \(\newcommand{\len}[1]{\left|#1\right|}\) \(\newcommand{\bbar}{\overline{\bvec}}\) \(\newcommand{\bhat}{\widehat{\bvec}}\) \(\newcommand{\bperp}{\bvec^\perp}\) \(\newcommand{\xhat}{\widehat{\xvec}}\) \(\newcommand{\vhat}{\widehat{\vvec}}\) \(\newcommand{\uhat}{\widehat{\uvec}}\) \(\newcommand{\what}{\widehat{\wvec}}\) \(\newcommand{\Sighat}{\widehat{\Sigma}}\) \(\newcommand{\lt}{<}\) \(\newcommand{\gt}{>}\) \(\newcommand{\amp}{&}\) \(\definecolor{fillinmathshade}{gray}{0.9}\)In Sections G.1 and G.2 we suggest topics that are related to the material in Chapter 1. Section G.3 supplements biological examples in Chapters 3 and 4. The material in G.4 supplements examples in Chapter 7 and provides additional practice with optimization. The optimal foraging time for a specific patch function studied in Chapter 7 is generalized in Section G.5. Section G.6 extends the study of trigonometric functions and their derivatives as seen in Chapter 15 to differential equations.
G.1 Michaelis-Menten transformed to a linear relationship
Michaelis-Menten kinetics explored in Equation (1.8) is a nonlinear saturating function in which the concentration \(x\) is the independent variable on which the reaction velocity, \(v\) depends:
\[v=\frac{K x}{k_{n}+x} . \nonumber \]
As discussed in Section 1.5, the constants \(K\) and \(k_{n}\) depend on the enzyme and are often quantified in a biochemical assay of enzyme action. Historically, a convenient way to estimate the values of \(K\) and \(k_{n}\) was to measure \(v\) for many different values of the initial substrate concentration. Without nonlinear fitting software widely available, Equation (1.8) was transformed (meaning that it was rewritten) as a linear relationship.
We can do so as well with algebra. We begin by taking reciprocals of our equation and expanding:
\[\begin{aligned} \frac{1}{v} & =\frac{k_{n}+x}{K x}, \\ & =\frac{k_{n}}{K x}+\frac{x}{K x} \\ & =\left(\frac{k_{n}}{K}\right) \frac{1}{x}+\left(\frac{1}{K}\right) \end{aligned} \nonumber \]
This suggests defining the two constants:
\[m=\frac{k_{n}}{K}, \quad b=\frac{1}{K} . \nonumber \]
In which case, the relationship between \(1 / v\) and \(1 / x\) becomes linear:
\[\left[\frac{1}{v}\right]=m\left[\frac{1}{x}\right]+b . \nonumber \]
Both the slope, \(m\) and intercept \(b\) of the straight line provide information about the parameters. The relationship in Equation (G.1), which is a disguised variant of Michaelian kinetics, is called the Lineweaver-Burk relationship. In Exercise 30 this is used to estimate the values of \(K\) and \(k_{n}\) from biochemical data about an enzyme.
G.2 Spacing of fish in a school
Many animals live or function best when they are in a group. Social groups include herds of wildebeest, flocks of birds, and schools of fish, as well as swarms of insects. Life in a group can affect the way that individuals forage (search for food), their success at detecting or avoiding being eaten by a predator, and other functions such as mating, protection of the young, etc. Biologists are interested in the ecological implications of groups on their own members or on other species with whom they interact, and how individual behavior, combined with environmental factors and random effects affect the shape, spacing and function of the groups.
In many social groups, the spacing between individuals is relatively constant from one part of the formation to another, because animals that get too close start to move away from one another, whereas those that get too far apart are attracted back. These spacing distances can be observed in a variety of groups, and were described in many biological publications. For example, Emlen [Emlen Jr, 1952] studied flocks of birds and found that gulls are spaced at about one body length apart. Similarly, Conder [J., 1949] observed a \(2-3\) body lengths spacing distance in tufted ducks while Miller [R.S. and J.D., 1966] found that in the flock he observed, sandhill cranes try to keep about \(5.8 \mathrm{ft}\) apart.
To explain why certain spacing is maintained in a group of animals, it was proposed that there are mutual attraction and repulsion interactions (effectively acting like simple forces) between individuals. Breder [Breder, 1954] followed a number of species of fish that school, and measured the individual spacing in units of the fish body length, showing that individuals are separated by \(0.16-0.25\) body length units. He suggested that the effective forces between individuals were similar to inverse power laws for repulsion and attraction. Breder considered a quantity he called cohesiveness, defined as:
\[c=\frac{A}{x^{m}}-\frac{R}{x^{n}}, \nonumber \]
where \(A, R\) are magnitudes of attraction and repulsion, \(x\) is the distance between individuals, and \(m, n\) are integer powers that govern how quickly the interactions fall off with distance. We could re-express the formula in Equation (G.2) as
\[c=A x^{-m}-R x^{-n} \nonumber \]
Thus, the function shown in Breder’s cohesiveness formula is related to our power functions, but the powers are negative integers. A specific case considered by Breder was \(m=0, n=2\), i.e. constant attraction and inverse square law repulsion,
\[c=A-\left(R / x^{2}\right) \nonumber \]
Breder specifically considered the "point of neutrality", where \(c=0\). The distance at which this occurs is:
\[x=(R / A)^{1 / 2} \nonumber \]
where attraction and repulsion are balanced. This is the distance at which two fish would be most comfortable: neither tending to move apart, nor get closer together.
G.3 A biological speed machine
Lysteria monocytogenes is a parasite that lives inside cells of the host, causing a nasty infection. It has been studied by cellular biologists for its amazingly fast propulsion, which uses the host’s actin filaments as "rocket fuel". Actin is part of the structural component of all animal cells, and is known to play a major role in cell motility. Lysteria manages to "hijack" this cellular mechanism, assembling it into its own comet tail, which it uses to propel inside the cell and pass from one cell to the next. Figure G.1 illustrates part of these curious traits.

Researchers in cell biology use Lysteria to learn about motility at the cellular level. It has been discovered that certain proteins on the external surface of this parasite (ActA) are responsible for the ability of Lysteria to assemble an actin filament tail. Surprisingly, even small plastic beads artificially coated in Lysteria’s ActA proteins can perform the same "trick": they assemble an actin tail which pushes the bead like a tiny rocket.
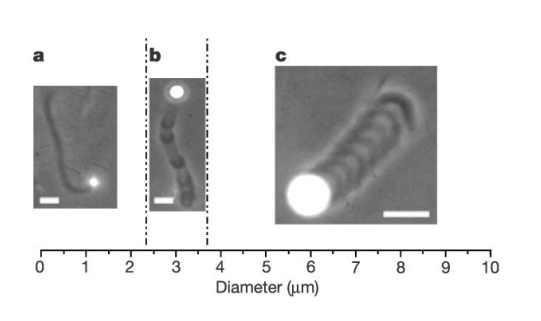
In a recent paper, Bernheim-Groswasser et al. [Bernheim-Groswasser et al., 2002] describe the motion of these beads, shown in Figure G.2. When the position of the bead is plotted on a graph with time as the horizontal axis, (see Figure G.3) we find that the trajectory is not a simple one: it appears that the bead slows down periodically, and then accelerates.

With the techniques developed in Chapters 3 and 4 , we can analyze the experimental data shown in Figure G.3 to determine both the average velocity of the beads, and the instantaneous velocity over the course of the motion.
Average velocity of the bead. We can get a rough idea of how fast the microbeads are moving by computing an average velocity over the time interval shown on the graph. We can use two (approximate) data points \((t, D(t))\), at the beginning and end of the run, for example \((45,20)\) and \((80,35)\) : the average velocity is
\[\begin{gathered} \bar{v}=\frac{\Delta D}{\Delta t} \\ \bar{v}=\frac{35-20}{80-45} \approx 0.43 \mu \mathrm{min}^{-1} \end{gathered} \nonumber \]
so the beads move with average velocity \(0.43\) microns per minute.
Units.
One micron is \(10^{-6}\) meters.
The changing instantaneous velocity
Because the actual data points are taken at finite time increments, the curve shown in Figure G.3 is not smooth. We smoothen it, as shown in Figure G.4 for a simpler treatment. In Figure G.5 we sketch this curve together with a collection of lines that represent the slopes of tangents along the curve. A horizontal tangent has slope zero: this means that at all such points (also indicated by the arrows for emphasis), the velocity of the beads is zero. Between these spots, the bead has picked up speed and moved forward until the next time in which it stops.


We show the velocity \(v(t)\), which is the derivative of the original function \(D(t)\) in Figure G.6. As shown here, the velocity has periodic increases and decreases.
G.4 Additional examples of geometric optimization
Rectangular box with largest surface area
We consider two examples of optimization where volumes, lengths, and/or surface areas are considered.
A box with square base and arbitrary height has string tied around each of its perimeter. The total length of string so used is 10 inches. Find the dimensions of the box with largest surface area, i.e. determine the largest amount of wrapping paper needed to wrap this box.
Solution

The total length of string is shown in Figure G.7. It consists of three perimeters of the box is as follows:
\[L=2(x+x)+2(x+y)+2(x+y)=8 x+4 y=10 . \nonumber \]
This total length is to be kept constant, so this equation is the constraint in this problem. This means that \(x\) and \(y\) are related to one another. We use this fact to eliminate one of them from the formula for surface area.
The surface area of the box is
\[S=4(x y)+2 x^{2} \nonumber \]
since there are two faces (top and bottom) which are squares (area \(x^{2}\) ) and four rectangular faces with area \(x y\). At the moment, the total surface area \(S\) is expressed in terms of both variables. Suppose we eliminate \(y\) from \(S\) by rewriting the constraint in the form:
\[y=\frac{5}{2}-2 x . \nonumber \]
Then
\[S(x)=4 x\left(\frac{5}{2}-2 x\right)+2 x^{2}=10 x-8 x^{2}+2 x^{2}=10 x-6 x^{2} . \nonumber \]
We show the shape of this function in Figure G.8. Note that \(S(x)=0\) at \(x=0\) and at \(10-6 x=0\) (which occurs at \(x=5 / 3\) ).

Since \(S\) is now expressed as a function of one variable, we can find its critical points by setting \(S^{\prime}(x)=0\), i.e., solving
\[S^{\prime}(x)=10-12 x=0 \nonumber \]
for \(x\) : we get \(x=10 / 12=5 / 6\). To find the corresponding value of \(y\) we substitute our result back into the constraint. This results in
\[y=\frac{5}{2}-2\left(\frac{5}{6}\right)=\frac{15-10}{6}=\frac{5}{6} . \nonumber \]
Thus the dimensions of the box of interest are all the same, i.e. it is a cube with side length \(5 / 6\).
We can verify that
\[S^{\prime \prime}(x)=-12<0, \nonumber \]
(indeed this holds for all \(x\) ), which means that \(x=5 / 6\) is a local maximum.
Further, we can find that
\[S=4\left(\frac{5}{6}\right)\left(\frac{5}{6}\right)+2\left(\frac{5}{6}\right)^{2}=\frac{25}{6} \nonumber \]
square inches, the maximum surface area of a box with such a constraint. Figure G.8 shows how the surface area varies as the dimension \(x\) of the box is varied.
A cylinder in a sphere
Find the cylinder of maximal volume that would fit inside a sphere of radius \(R\).
Solution
We sketch a cylinder inside a sphere as in Figure G.9.

It is helpful to add the radius of the sphere and of the cylinder. We define the following:
\[\begin{aligned} h & =\text { height of cylinder, } \\ r & =\text { radius of cylinder, } \\ R & =\text { radius of sphere. } \end{aligned} \nonumber \]
Then \(R\) is assumed a given fixed positive constant, and \(r\) and \(h\) are dimensions of the cylinder to be determined.
From Figure G.9 we see that the cylinder fits if the top and bottom rims touch the circle. When this occurs, the dark line in Figure G.9 is a radius of the sphere, and so has length \(R\).
The connection between the variables (our constraint) is given from Pythagoras’ theorem by:
\[R^{2}=r^{2}+\left(\frac{h}{2}\right)^{2} . \nonumber \]
We maximize the volume of the cylinder,
\[V=\pi r^{2} h \nonumber \]
subject to the above constraint.
Eliminating \(r^{2}\) using the Pythagoras theorem leads to
\[V(h)=\pi\left(R^{2}-\frac{h^{2}}{4}\right) h . \nonumber \]
We see that the problem is very similar to the previous discussion. The reader can show by working out the steps that
\[V^{\prime}(h)=0 \nonumber \]
occurs at the critical point
\[h=\frac{2}{\sqrt{3}} R \nonumber \]
and this is a local maximum.
G.5 Optimal foraging with other patch functions
In Section 7.4, we computed an optimal foraging time for a specific patch function \(f(t)\) given by Equation (7.6). However, we can gain insight and obtain an interesting result without making this assumption. We now consider a similar analysis with a more general example.
Carry out the calculations for the optimal value patch residence time for a general patch energy function \(f(t)\), without using the formula Equation (7.6).
Solution
We use the expression for \(R(t)\) given by Equation (7.7). Differentiating, we find the first derivative,
\[R^{\prime}(t)=\frac{f^{\prime}(t)(\tau+t)-f(t)}{(\tau+t)^{2}}=\frac{G(t)}{H(t)} \nonumber \]
where
\[G(t)=f^{\prime}(t)(\tau+t)-f(t), \quad H(t)=(\tau+t)^{2} . \nonumber \]
(The calculation is easier with this notation.) To maximize \(R(t)\) we set
\[R^{\prime}(t)=0 \nonumber \]
which can occur only when the numerator of the above equation is zero, i.e.
\[G(t)=0 . \nonumber \]
This means that
\[f^{\prime}(t)(\tau+t)-f(t)=0 \nonumber \]
so that, after simplifying algebraically,
\[f^{\prime}(t)=\frac{f(t)}{\tau+t} . \nonumber \]
A geometric argument. In practice, we need to specify a function for \(f(t)\) in order to solve for the optimal time \(t\). However, we can also solve this problem using a geometric argument.
Eqn (G.3) equates two quantities that can be interpreted as slopes. On the right is the slope of a tangent line. On the left is the slope (rise over run) of some right triangle whose height is \(f(t)\) and whose base length is \(\tau+t\). In Figure G.10, we show each slope on its own: in the left panel, \(f^{\prime}(t)\) is the slope of the tangent line to the graph of \(f(t)\). In the central panel, we have constructed some triangle with the property that its hypotenuse has slope \(f(t) /[\tau+t]\). On the right panel we have superimposed both, selecting a value of \(t\) for which the slope of the triangle is the same as the slope of the tangent line.

Notice that in order to fit the triangle on the same diagram, we had to place its tip at the point \(-\tau\) along the horizontal axis. When these slopes coincide, it means that we have satisfied Equation (G.3), and found the desired time \(t\) for optimal foraging.
We can use this observation to come up with the following steps to solve Figure G.10: The solution to the optimal foraging problem can be expressed geometrically in the form shown in this figure. The tangent line at the (optimal) time \(t\) should have the same slope as the hypotenuse of the right triangle shown above. The diagram on the far right is sometimes termed the "rooted tangent" diagram. an optimal foraging problem in general:
- A biologist conducts some field experiments to determine the mean travel time from food to nest, \(\tau\), and the shape of the energy gain function \(f(t)\).
Note: this may require capturing the animal and examining the contents of its stomach. We leave this task to our biological colleagues.
- We draw a sketch of \(f(t)\) as shown in rightmost panel of Figure G.10 and extend the \(t\) axis in the negative direction. At the point \(-\tau\) we draw a line that just touches the curve \(f(t)\) at some point (i.e. a tangent line). The slope of this line is \(f^{\prime}(t)\) for some value of \(t\).
- The value of \(t\) at the point of tangency is the optimal time to spend in the patch!
The diagram drawn in our geometric solution (right panel in Figure G.10) is often called a "rooted tangent".
We have shown that the point labeled \(t\) indeed satisfies the condition that we derived above for \(R^{\prime}(t)=0\), and hence is a critical point.
Checking the type of critical point
We still need to show that this solution leads to a maximum efficiency, (rather than, say a minimum or some other critical point). We do this by examining \(R^{\prime \prime}(t)\).
Recall that
\[R^{\prime}(t)=\frac{G(t)}{H(t)} \nonumber \]
in terms of the notation used above. Then
\[R^{\prime \prime}(t)=\frac{G^{\prime}(t) H(t)-G(t) H^{\prime}(t)}{H^{2}(t)} . \nonumber \]
But, according to our remark above, at the patch time of interest (the candidate for optimal time),
\[G(t)=0 \nonumber \]
so that
\[R^{\prime \prime}(t)=\frac{G^{\prime}(t) H(t)}{H^{2}(t)}=\frac{G^{\prime}(t)}{H(t)} . \nonumber \]
We substitute the derivative of \(G^{\prime}(t), H(t)\) into this ratio:
\[\begin{aligned} G(t)=f^{\prime}(t)(\tau+t)-f(t) \Rightarrow G^{\prime}(t) & =f^{\prime \prime}(t)(\tau+t)+f^{\prime}(t)-f^{\prime}(t) \\ & =f^{\prime \prime}(t)(\tau+t) \end{aligned} \nonumber \]
We find that
\[R^{\prime \prime}(t)=\frac{f^{\prime \prime}(t)(\tau+t)}{(\tau+t)^{2}}=\frac{f^{\prime \prime}(t)}{(\tau+t)} . \nonumber \]
The denominator of this expression is always positive, so the sign of \(R^{\prime \prime}(t)\) is the same as the sign of \(f^{\prime \prime}(t)\). But in order to have a maximum efficiency at some residence time, we need \(R^{\prime \prime}(t)<0\). This tells us that the gain function has to have the property that \(f^{\prime \prime}(t)<0\), i.e. has to be concave down at the optimal residence time.
Returning to some of the shapes of the function \(f(t)\) that we saw in Figure 7.7, we see that only some of these lead to an optimal solution. In cases (1), (2), (4) the function \(f(t)\) has no points of downwards concavity on its graph. This means that in such cases there is no local maximum. The optimal efficiency would then be attained by spending as much time as possible in just one patch, or as little time as possible in any patch, i.e. it would be attained at the endpoints.
G.6 Trigonometric functions and differential equations
As we saw in Chapter 15 , the functions \(\sin (t)\) and \(\cos (t)\) are related to one another via differentiation: one is the derivative of the other (with a multiple of the factor \((-1))\) :
\[\frac{d \sin (t)}{d t}=\cos (t), \quad \frac{d \cos (t)}{d t}=-\sin (t) . \nonumber \]
The connection becomes even clearer when we examine the second derivatives of these functions:
\[\frac{d^{2} \sin (t)}{d t^{2}}=\frac{d \cos (t)}{d t}=-\sin (t), \quad \frac{d^{2} \cos (t)}{d t^{2}}=-\frac{d \sin (t)}{d t}=-\cos (t) . \nonumber \]
Thus, for each of the functions \(y=\sin (t), y=\cos (t)\), we find that the function and its second derivative are related to one another by the differential equation (DE) \(d^{2} y / d t^{2}=-y\). Here the highest derivative is a second derivative, and we denote this a second order DE.
More generally, we make the following observations:
The functions
\[x(t)=\cos (\omega t), \quad y(t)=\sin (\omega t) \nonumber \]
satisfy a pair of differential equations,
\[\frac{d x}{d t}=-\omega y, \quad \frac{d y}{d t}=\omega x . \nonumber \]
The functions
\[x(t)=\cos (\omega t), \quad y(t)=\sin (\omega t) \nonumber \]
also satisfy a related differential equation with a second derivative
\[\frac{d^{2} x}{d t^{2}}=-\omega^{2} x . \nonumber \]
These follow by the same reasoning, where the chain rule is applied in differentiation.
Students of physics may recognize the equation that governs the behavior of a harmonic oscillator, and see the connection between the circular motion of our point on the circle, and the differential equation for periodic motion.